. Introduction
. A brief overview of the family Grimmiaceae in South America
The family Grimmiaceae is well represented in South America in terms of species richness and frequency of occurrence. Its members primarily colonize dry, exposed rocky habitats, which are widespread along the Andean chain, extending from Tierra del Fuego in the south to Colombia and Venezuela in the north. In South America, the family comprises 65 species, traditionally assigned to four broadly circumscribed genera: Grimmia Hedw., Racomitrium Brid., Schistidium Bruch & Schimp., and Coscinodon Spreng. Traditionally, the genera Scouleria Hook., Aligrimmia R.S. Williams, Coscinodontella R.S. Williams, Jaffueliobryum Thér., and Ptychomitrium were also included in the Grimmiaceae (Williams, 1903, 1927; Brotherus, 1924; Deguchi, 1987; Thériot, 1928). Of these, Scouleria is now placed in a separate family, Scouleriaceae (Churchill, 1981), whereas the remaining four genera are currently assigned to Ptychomitriaceae (Murray, 1984; Hernández-Maqueda et al., 2008b).
The genus Grimmia includes 21 species in South America, occurring mainly in the Andean countries and rarely in southeastern Brazil, Uruguay, and the Falkland Islands (Muñoz, 1999). It is a heterogeneous genus whose species show considerable morphological diversity, and many authors (e.g., Buysson, 1883; Churchill, 1981; Cao & Vitt, 1986; Muñoz, 1998) have regarded it as an unnatural polyphyletic taxon. This has provided the basis for splitting it into several segregates that are well circumscribed by combinations of gametophytic and sporophytic characters (Ochyra et al., 2003). The validity of this approach has also been supported by molecular studies, which recover these segregates as distinct clades (Streiff, 2006; Hernández-Maqueda et al., 2008a; Solano et al., 2023).
Likewise, the broadly circumscribed genus Racomitrium, which comprises 21 species in South America and shows a distribution pattern similar to that of Grimmia (Ochyra et al., 1988, 2015; Bednarek-Ochyra & Ochyra, 1994, 2003, 2010, 2011, 2012a; Bednarek-Ochyra et al., 1999; Ellis et al., 2011; Bednarek-Ochyra & Plášek, 2017), is also heterogeneous. It includes at least five distinct genera that form discrete entities without morphological intergradation and can be clearly delimited by unique sets of morphological and anatomical characters, in agreement with the molecular evidence (Ochyra et al., 2003; Bednarek-Ochyra et al., 2014, 2015; Sawicki et al., 2015). The smallest genus of grimmialean mosses on the continent is Coscinodon, which includes only four species (Hastings, 1996, 1999; Ochyra, 2004a).
. A brief survey of studies on Schistidium in the Southern Hemisphere
The most problematic and controversial issue concerns the assessment of species richness within the genus Schistidium in South America. Although this is one of the oldest moss genera, recognized as early as 1819 (Bridel, 1819), and represents a distinct and readily distinguishable taxon, it has a complex and somewhat unsettled nomenclatural and taxonomic history. Since the adoption of the Tokyo Code (Greuter et al., 1994), the generic name has been treated as nomen conservandum, with the conserved type S. maritimum (Sm. ex R. Scott) Bruch & Schimp. (Ochyra & Isoviita, 1989). This decision reflects the fact that Schistidium sensu Bridel (1819) was misapplied: its original generitype, S. pulvinatum (Hedw.) Brid. (Mårtensson, 1956), was later shown to be conspecific with Grimmia anodon Bruch & Schimp., thereby rendering Schistidium congeneric with Grimmia (Ochyra, 1989a).
The modern concept of Schistidium was first outlined in the Bryologia europaea (Bruch et al., 1845). Only three species were included in this newly recircumscribed genus: S. maritimum, S. confertum (Funck) Bruch & Schimp., and S. apocarpum (Hedw.) Bruch & Schimp. The latter species, however, was interpreted very broadly, with the names of nearly all previously described European species and varieties treated as synonyms of its name. Only three particularly distinct species described earlier were recognized as varieties or subvarieties of S. apocarpum. Because Bryologia europaea was regarded as the ultimate authority on moss taxonomy and nomenclature in Europe, this treatment of species within Schistidium had a profoundly negative impact on the systematics of the genus, not only in Europe, but also elsewhere. Researchers working on this genus recognized the extensive morphological variability of S. apocarpum; however, they interpreted its diverse phenotypes as numerous varieties, forms, or ecomorphs within a single species (Podpěra, 1954). This approach was adopted not only in Europe but, initially, also in other parts of the world. For example, Schistidium specimens reported from Tierra del Fuego, the Falkland Islands, and Îles Kerguelen (Wilson & Hooker, 1847), New Zealand (Wilson, 1854; Hooker, 1867), and Tasmania (Wilson, 1859) were treated as varieties of Grimmia apocarpa Hedw., although no formal varietal names were assigned to them. In the later decades of the nineteenth century and the first half of the twentieth century, exotic Schistidium specimens were typically described as separate species, most often under the genus Grimmia (e.g., Hampe, 1860; Mitten, 1869; Müller, 1883, 1889, 1890, 1898a, 1898b, 1899; Röll, 1890; Brown, 1895, 1903; Herzog, 1916). However, most of these taxa have not been critically examined from a taxonomic perspective, and their true status remains uncertain.
The culmination of this broad interpretation of Schistidium apocarpum was the taxonomic revision of Schistidium published by Bremer (1980a, 1980b, 1981), in which the names of more than 140 species and infraspecific taxa were reduced to synonyms of S. apocarpum. As a result, the species became a heterogeneous assemblage of taxa that could neither be clearly defined nor convincingly maintained as a single species. Consequently, determining the species richness of Schistidium remains difficult in most regions outside Europe, North America, and northern Asia.
The turning point in the history of systematic research on the genus Schistidium was the publication of a completely different, revolutionary concept of the S. apocarpum complex in Scandinavia, based on numerous collections from continental Europe, northern Asia, and North America north of Mexico (Blom, 1996, 1998). The most important aspect of this monograph was, above all, the typification and precise recircumscription of the core species of this complex, namely, S. apocarpum itself. This species has its main center of occurrence in northern and central Europe, extending southward to the northern margins of the Mediterranean region, with an isolated locality in Madeira, and eastward to the Caucasus and the Ural Mountains, with isolated occurrences extending into Central Siberia (Blom, 1996). In North America, however, S. apocarpum occurs relatively rarely and in a scattered manner across the northern part of the continent, from Newfoundland in the east to Alaska and British Columbia in the west, with its southern range limit running through the northern states of the United States (Maine, Vermont, Michigan, Wisconsin, and Washington) (McIntosh, 2007). To date, its occurrence has not been confirmed in the Southern Hemisphere, tropics, or southern Asia, although the genus in these regions requires detailed taxonomic study.
To date, the only regions at the southern extremity of the Earth in which the genus Schistidium has undergone taxonomic revision are subantarctic South Georgia (Bell, 1984; Ochyra et al., 2002a) and Antarctica (Ochyra, 2004b; Ochyra et al., 2008a, 2008b). In the latter region, Schistidium comprises 13 species and is the most species-rich genus on the continent. Of these, five species have been described as new to science and are endemic to Antarctica (Ochyra, 1987a, 1998a, 2003, 2004c; Ochyra et al., 2003). In other extra-Holarctic regions, the traditional concept of S. apocarpum is still widely applied, which precludes an accurate assessment of the true diversity of this genus, for example, in New Zealand (Fife, 2000; Gibb et al., 2018; Allan Herbarium, 2023), Australia (Klazenga, 2012), Central America (Allen, 2002), and southern Africa (Magill, 1981).
The oldest specimens of Schistidium from the Southern Hemisphere date back to the early 1840s and were collected by the distinguished British botanist Joseph Dalton Hooker (1817–1911). Between 1839 and 1843, he served as a surgeon-botanist aboard HMS Erebus in James Clark Ross’s famous Antarctic expedition (Hooker, 1847). The first, and at the same time the oldest, specimens were collected in the subantarctic Îles Kerguelen archipelago, where the expedition stopped on 12 May and remained until 20 July 1840. Hooker collected two species: S. falcatum (Hook.f. & Wilson) B. Bremer, which was originally described as Grimmia falcata Hook.f. & Wilson as the first species of Schistidium from the Southern Hemisphere new to science (Hooker & Wilson, 1844) and S. apocarpum, within which two unnamed varieties were distinguished. These were described a few years later as a new species, Grimmia amblyophylla Müll.Hal. (Müller, 1849). It was subsequently transferred to the genus Schistidium as S. amblyophyllum (Müll.Hal.) Ochyra & Hertel (Ochyra & Hertel, 1990). Greene (1986) suggests that this combination was used by Herzog (1960). Indeed, he used this binomial but did not fulfill the requirements of Art. 41 of the ICN (Turland et al., 2025) for the valid publication of a name, which requires a clear citation of the basionym or replaced synonym with full bibliographic details.
The Antarctic expedition then stopped twice in Tasmania, from August 16 to November 12, 1840, and from April 7 to July 7, 1841, where Hooker collected two specimens that were identified as an unnamed variety with muticous and awnless leaves (Wilson, 1859). From Tasmania, the expedition proceeded to New Zealand, where it stayed from August 18 to November 15, 1841, in the Bay of Islands on the North Island, where Hooker collected one specimen that was again identified as an unnamed variety of Grimmia apocarpa (Wilson, 1854). Finally, the expedition travelled to the Western Hemisphere, where it remained in Berkeley Sound on East Falkland from April 6 to September 6, 1842, where Hooker collected one specimen identified as G. apocarpa var. 1 (Wilson & Hooker, 1847). From there, the expedition went to Hermite Island in the Tierra del Fuego archipelago, where Cape Horn is located, and stayed there from September 21 to mid-December 1842. Here, a specimen identified as G. apocarpa var. 4 was collected, which Müller (1849) described as a new species, G. amblyophylla. In addition, a second specimen was found and identified as G. maritima (Wilson & Hooker, 1847). This specimen certainly belongs to the S. apocarpum complex, but its identity, like that of all other specimens collected by J. D. Hooker during this Antarctic expedition, has not yet been determined. This species is not listed by Mitten (1869), but he reported S. apocarpum from Hermite Island, and it is highly probable that this record is based on the specimen originally identified as S. maritimum.
In the first half of the nineteenth century, only one additional specimen of Schistidium apocarpum from central Chile was reported from South America, which W. Ph. Schimper identified as an unnamed variety of this species with blunt, hairless leaves (Montagne, 1850). In the second half of that century, however, six new species were described from this region, five of which are still accepted today, including one from Peru (Sullivant, 1859), three from Ecuador (Mitten, 1869), and two from northwestern Argentina (Müller, 1882). The largest number, as many as 18 species, were described from South America during the first four decades of the twentieth century (Dusén, 1903, 1905; Cardot, 1908; Herzog, 1910, 1934, 1937; Williams, 1916; Brotherus, 1920; Cardot & Brotherus, 1923; Thériot, 1923), while one species was described from Chile shortly after World War II (Bartram, 1946). In the present century, only one new species has been described from Peru, S. deguchianum Ochyra & Bedn.-Ochyra (Ochyra & Bednarek-Ochyra, 2011), based on herbarium specimens collected in 1915. The species of Schistidium that have been described and recorded in South America are presented in chronological order in Table 1.
While checking the TROPICOS database (https://www.tropicos.org/name/35168048, accessed on 27 March 2026), our attention was drawn to a specimen determined as Schistidium cinclidodonteum (Müll.Hal.) B. Bremer, which was collected in 1977 by Pirkko and Eberhard Hegewald in Peru. This species was long considered endemic to the Pacific coast of North America, where it occurs from California to Washington and Idaho (McIntosh, 2007), but has recently also been found on the other side of the Atlantic, in Morocco (Ros et al., 2000), and on Gran Canaria in Macaronesia (Dirkse & Losada-Lima, 2019). Although a trans-American disjunction may seem unusual, it is a documented phenomenon. A pertinent example is the occurrence in Colombia of the amphipacific species Codriophorus mollis (Cardot) Bedn.-Ochyra & Ochyra, which is otherwise widely distributed in Pacific North America and the Far East of Asia (Bednarek-Ochyra, 2006). Another example is Syntrichia lithophila (Dusén) Ochyra R.H. Zander, a species widely distributed in Patagonia and western Antarctica (Saługa et al., 2022). It has subsequently been reported from Oregon (Brooks & Jáuregui-Lazo, 2023) and, more recently, from extreme northeastern California based on an unpublished collection by Jason R. Brooks housed in CAS (James R. Shevock, pers. comm., June 6, 2026).
It also cannot be ruled out that the Peruvian specimen was misidentified and actually represents Schistidium falcatum, a species occurring in the southern and central Andes in neighboring Bolivia, and in the far south extending into the maritime Antarctic and exhibiting an amphiatlantic disjunction, reaching eastward to the Kerguelen Province in the Subantarctic (Zanten, 1971; Bremer, 1980b; Ochyra & Bell, 1984; Ochyra et al., 2008b; Ellis et al., 2018). This is all the more likely because S. falcatum is highly similar to S. cinclidodonteum. A re-examination of this voucher specimen confirmed that it had indeed been misidentified, but that it was in fact identical to S. deguchianum. This species was previously found at a single locality in Peru and has now been rediscovered in the country.
. Material and methods
The description and illustration of Schistidium deguchianum are based on a single specimen collected in 1977 by Pirkko and Eberhard Hegewald in Peru, which was deposited in the bryophyte herbarium of the Missouri Botanical Garden (MO), St. Louis, USA. Gametophyte and sporophyte material was examined using standard bryological methods. The samples were rehydrated in water, sectioned, and examined using a Nikon SMZ-10A stereomicroscope and a Nikon Lobophot-2 compound microscope. Observations and measurements were made on materials mounted in Hoyer’s solution (Anderson, 1954). Transverse sections of the stems and leaves were prepared manually using a razor blade. Macro-photographs were taken using an Olympus SZ61 microscope, micro-photographs using an Olympus BX53F microscope, and SEM images using a JEOL scanning electron microscope. The map was created using a freely accessible base map from Google Maps and processed using CorelDRAW X3 (Corel Corporation).
The present study is based on an extensive examination of type specimens of all South American species of Schistidium deposited in the following herbaria: B, BM, BR, FH, H, HBG, JE, MO, NY, PC, S, and W. Herbarium acronyms follow Index Herbariorum (https://sweetgum.nybg.org/science/ih/; accessed 27 March 2026).
. Results and discussion
. Peruvian representation
The specimens of Schistidium deguchianum from the newly discovered locality closely matched the type specimen of this species (Figures 1–3). They are medium-sized, stiff, and rigid plants, forming rather dense tufts; brown with a blackish hue, often becoming brown-greenish or olivaceous at the tips of the branches and stems. The stems are 2–4 cm long, inflexible, and irregularly branched, densely and closely foliated above, but mostly denuded below, where they appear bristly due to erosion of the leaf laminae, except for the persistent, coarse, bristle-like costae. The stem bases are usually densely radiculose, with light-brown, mostly unbranched, and smooth rhizoids. In cross-section, the stem is circular and consists of a weak, uni- to partly bilayered cortex composed of small, substereid cells with small lumina and with incrassate, brown to yellowish-brown walls. This cortex is sharply demarcated from the 4–6 layers of large hyaline medullary cells. The central strand is large and distinct, comprising 30–50 small, thin-walled cells. Stem and branch leaves are similar in shape; they are erect and appressed, non-decurrent, and not or slightly altered, although the apices may sometimes become recurved upon drying. When wet, the leaves are erect-spreading, straight or slightly curved, alutaceous, very thick, lanceolate to ovate-lanceolate, and gradually taper to an acute apex, measuring (1.7–)1.9–2.8(–3.0) mm long and 0.5–0.9 mm wide. The leaves are concave below, becoming narrowly canaliculate to bluntly keeled toward the apex, and consistently lack a hair-point; the margins are plane and erect, entire throughout or bluntly and remotely serrulate, becoming lumpy or erose-sinuate near the apex, and only rarely sharply serrulate at the tip. The lamina is entirely bistratose in the median and proximal regions, and (2–)3–4-stratose distally, forming somewhat bulging marginal thickenings that are 3–6 cells wide. The costa is prominent, yellow to yellow-brownish, and sharply delimited from the laminal cells; percurrent, plano-convex, and semiterete to elliptical in cross-section, measuring 80–95 μm in width near the base and gradually narrowing upward to 50–70 μm wide near the apex; 4-stratose, with 5–6 dorsal and median cells forming a strong stereid band, and two rows of larger ventral cells visible in the transverse section. The laminal cells are smooth and rather opaque, bistratose throughout, with unistratose patches near the base and 3–4-stratose streaks in the distal portion. They are nearly homogeneous across the lamina, arranged in regular longitudinal rows, and vary in shape from rounded and transversely elliptical to rounded-quadrate, thin to moderately thick-walled, measuring 5–7 μm in length and 4–6 μm in width. In the basal region near the costa, they become more transparent and short-rectangular, measuring 6–8 μm in width and 12–20(–30) μm long. The basal marginal cells are undifferentiated.
Figure 1
Macro and micro photographs of Schistidium deguchianum taken from the specimen from Jauja Province in Peru: (a) habit, (b) perichaetium with a mature operculate capsule, (c) stem transverse section, (d) upper leaf cells, (e) mid-leaf cells, (f) basal juxtacostal cells, (g) basal cells in a leaf angle, (h-i) vegetative leaves, (j) leaf apex, (k-n) leaf cross-section, sequentially from apex to base. All data were obtained from MO 5143304. Scale bars: (a) 1 cm, (b) 2 mm, (c) 250 μm, (d-g, j) 50 μm, (h-i) 50 μm (k-n) 100 μm.
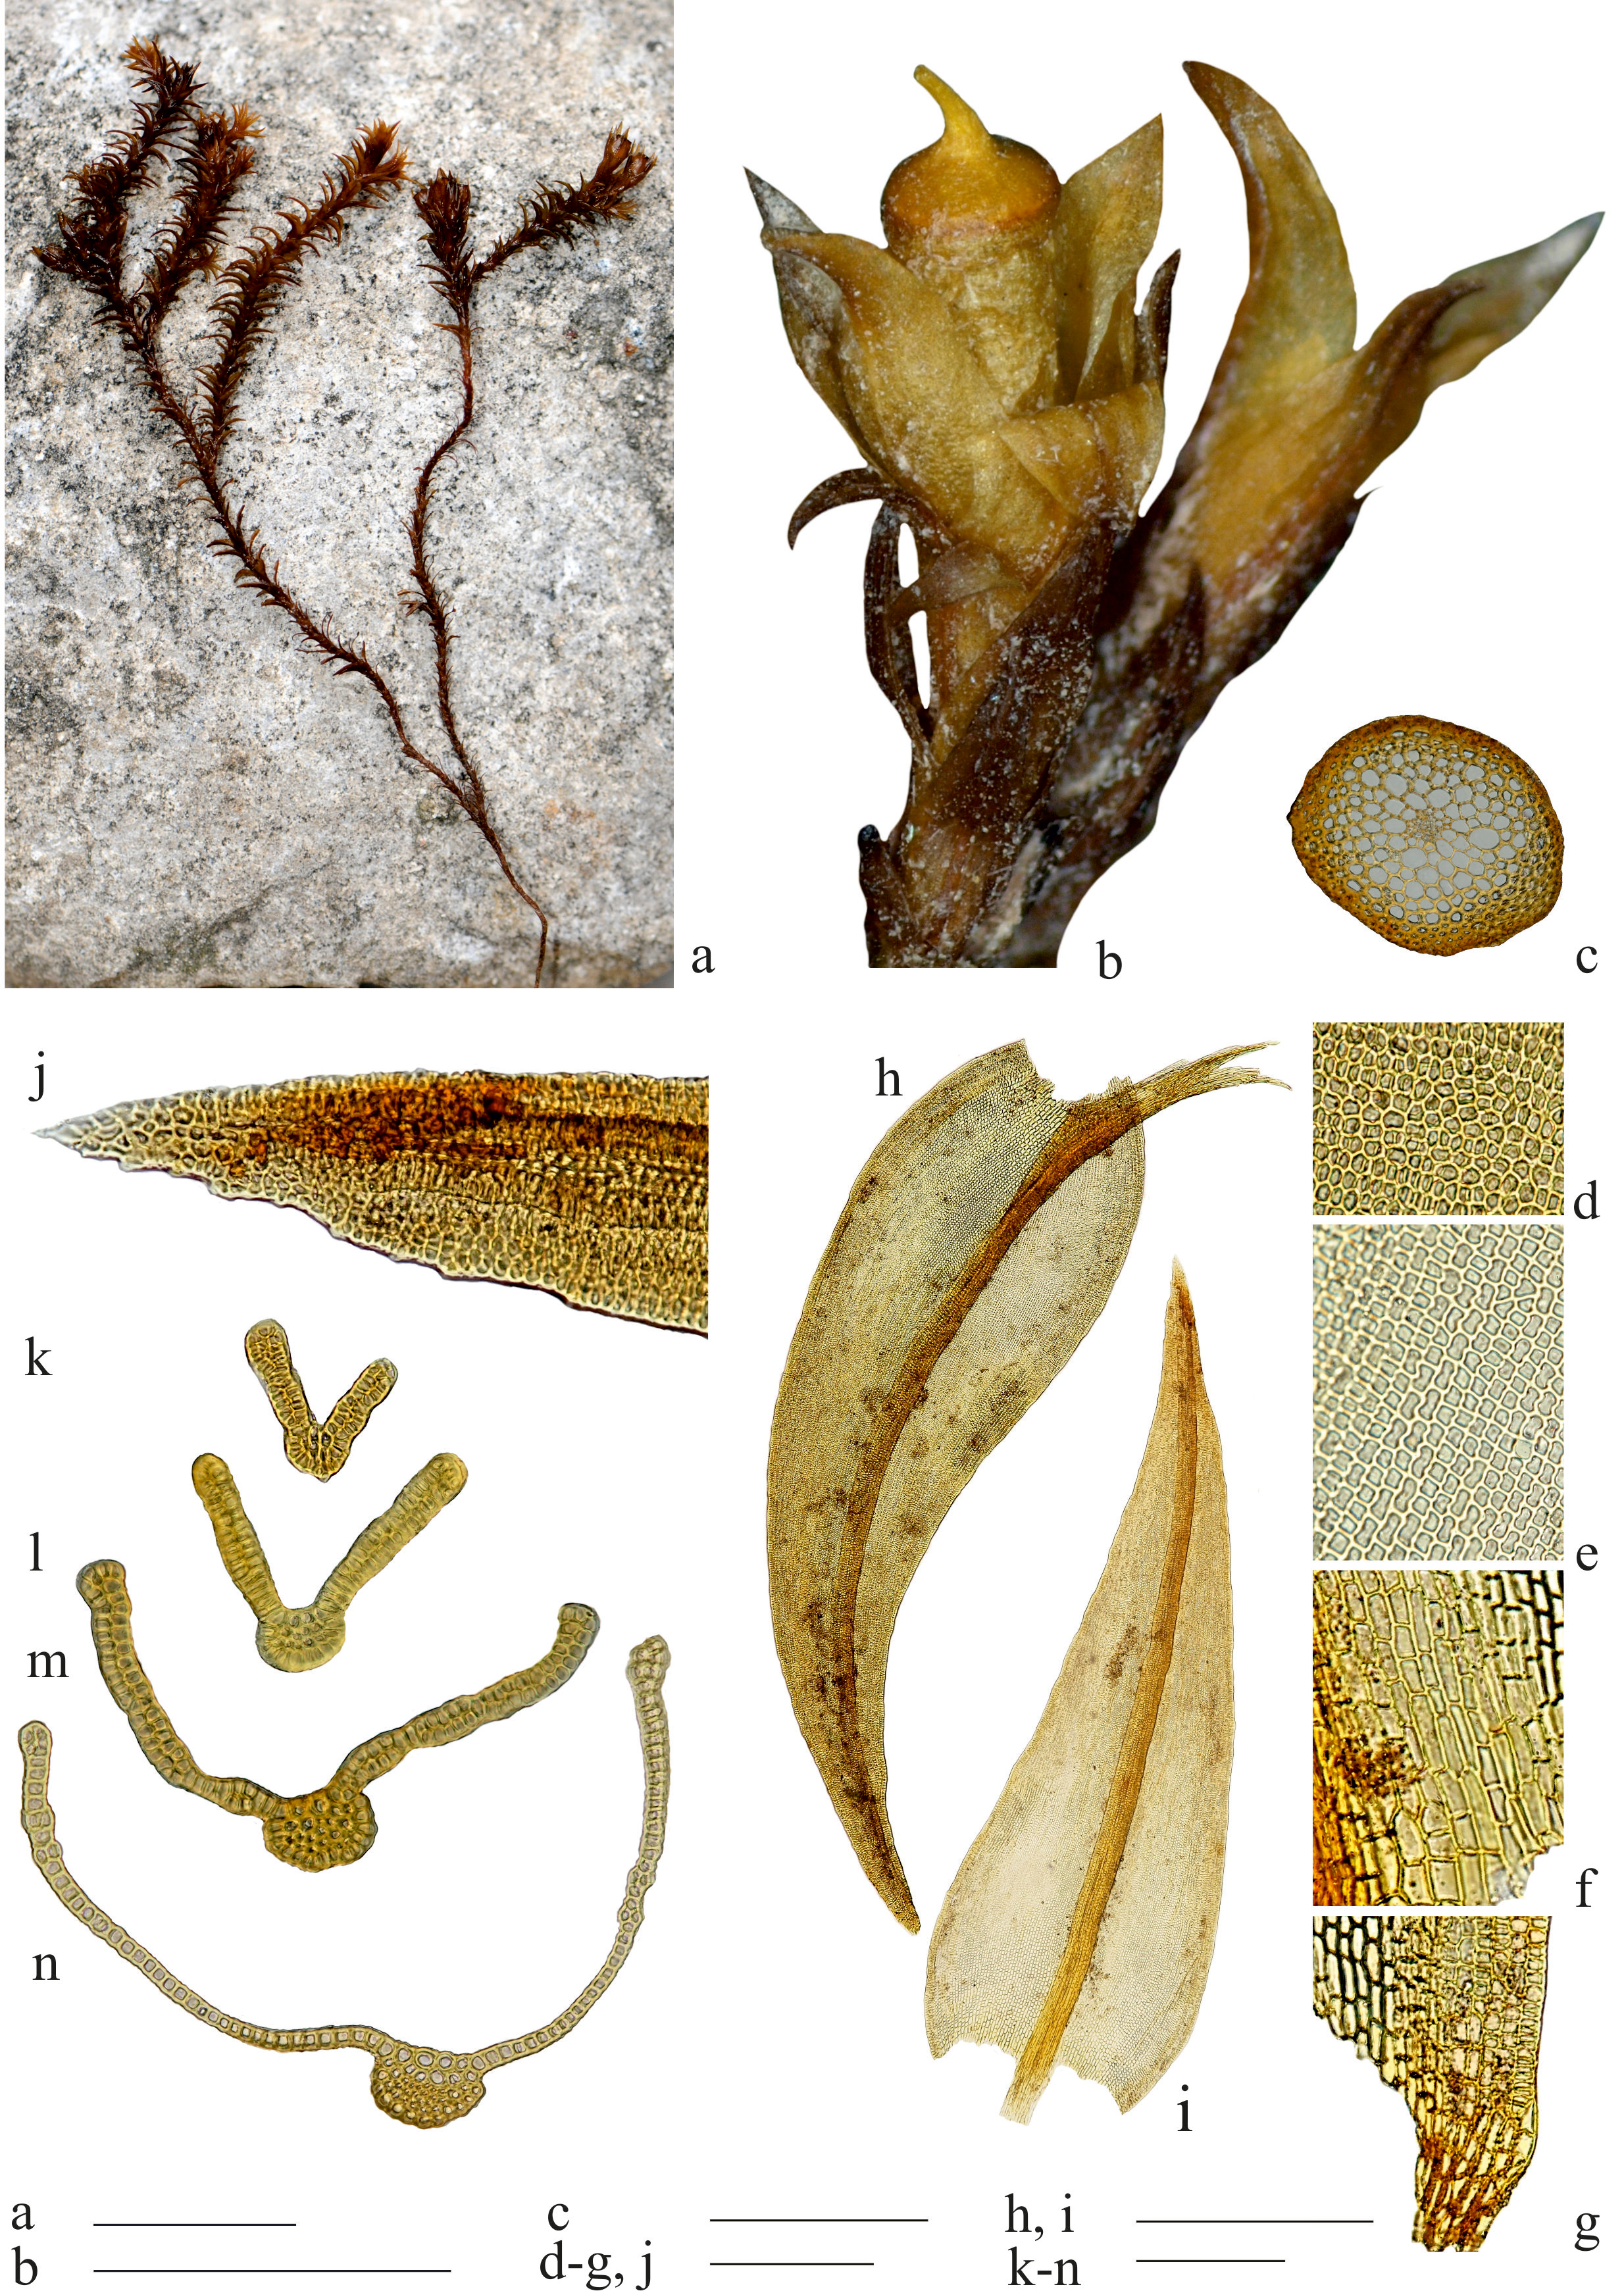
Figure 2
Macro- and micro-photographs of Schistidium deguchianum taken from the specimen from Jauja Province in Peru: (a) perichaetium with deoperculate capsules, (b) perichaetium with the perichaetial leaves removed, showing the capsule with the seta, (c) spores, (d-f) the outermost, meian, and innermost perichaetial leaves, (g) exothecial cells at the capsule mouth, (h) exothecial cells in the mid-urn, (i) exothecial cells above the base of the urn, (j) deoperculate capsule attached to the seta, (k) peristome teeth and exothecial cells in the upper part of the urn. All data were obtained from MO 5143304. Scale bars: (a) 2 mm, (b) 0.5 cm, (c) 20 μm, (d-f) 1 mm, (g-i) 50 μm, (j) 1 mm, (k) 40 μm.
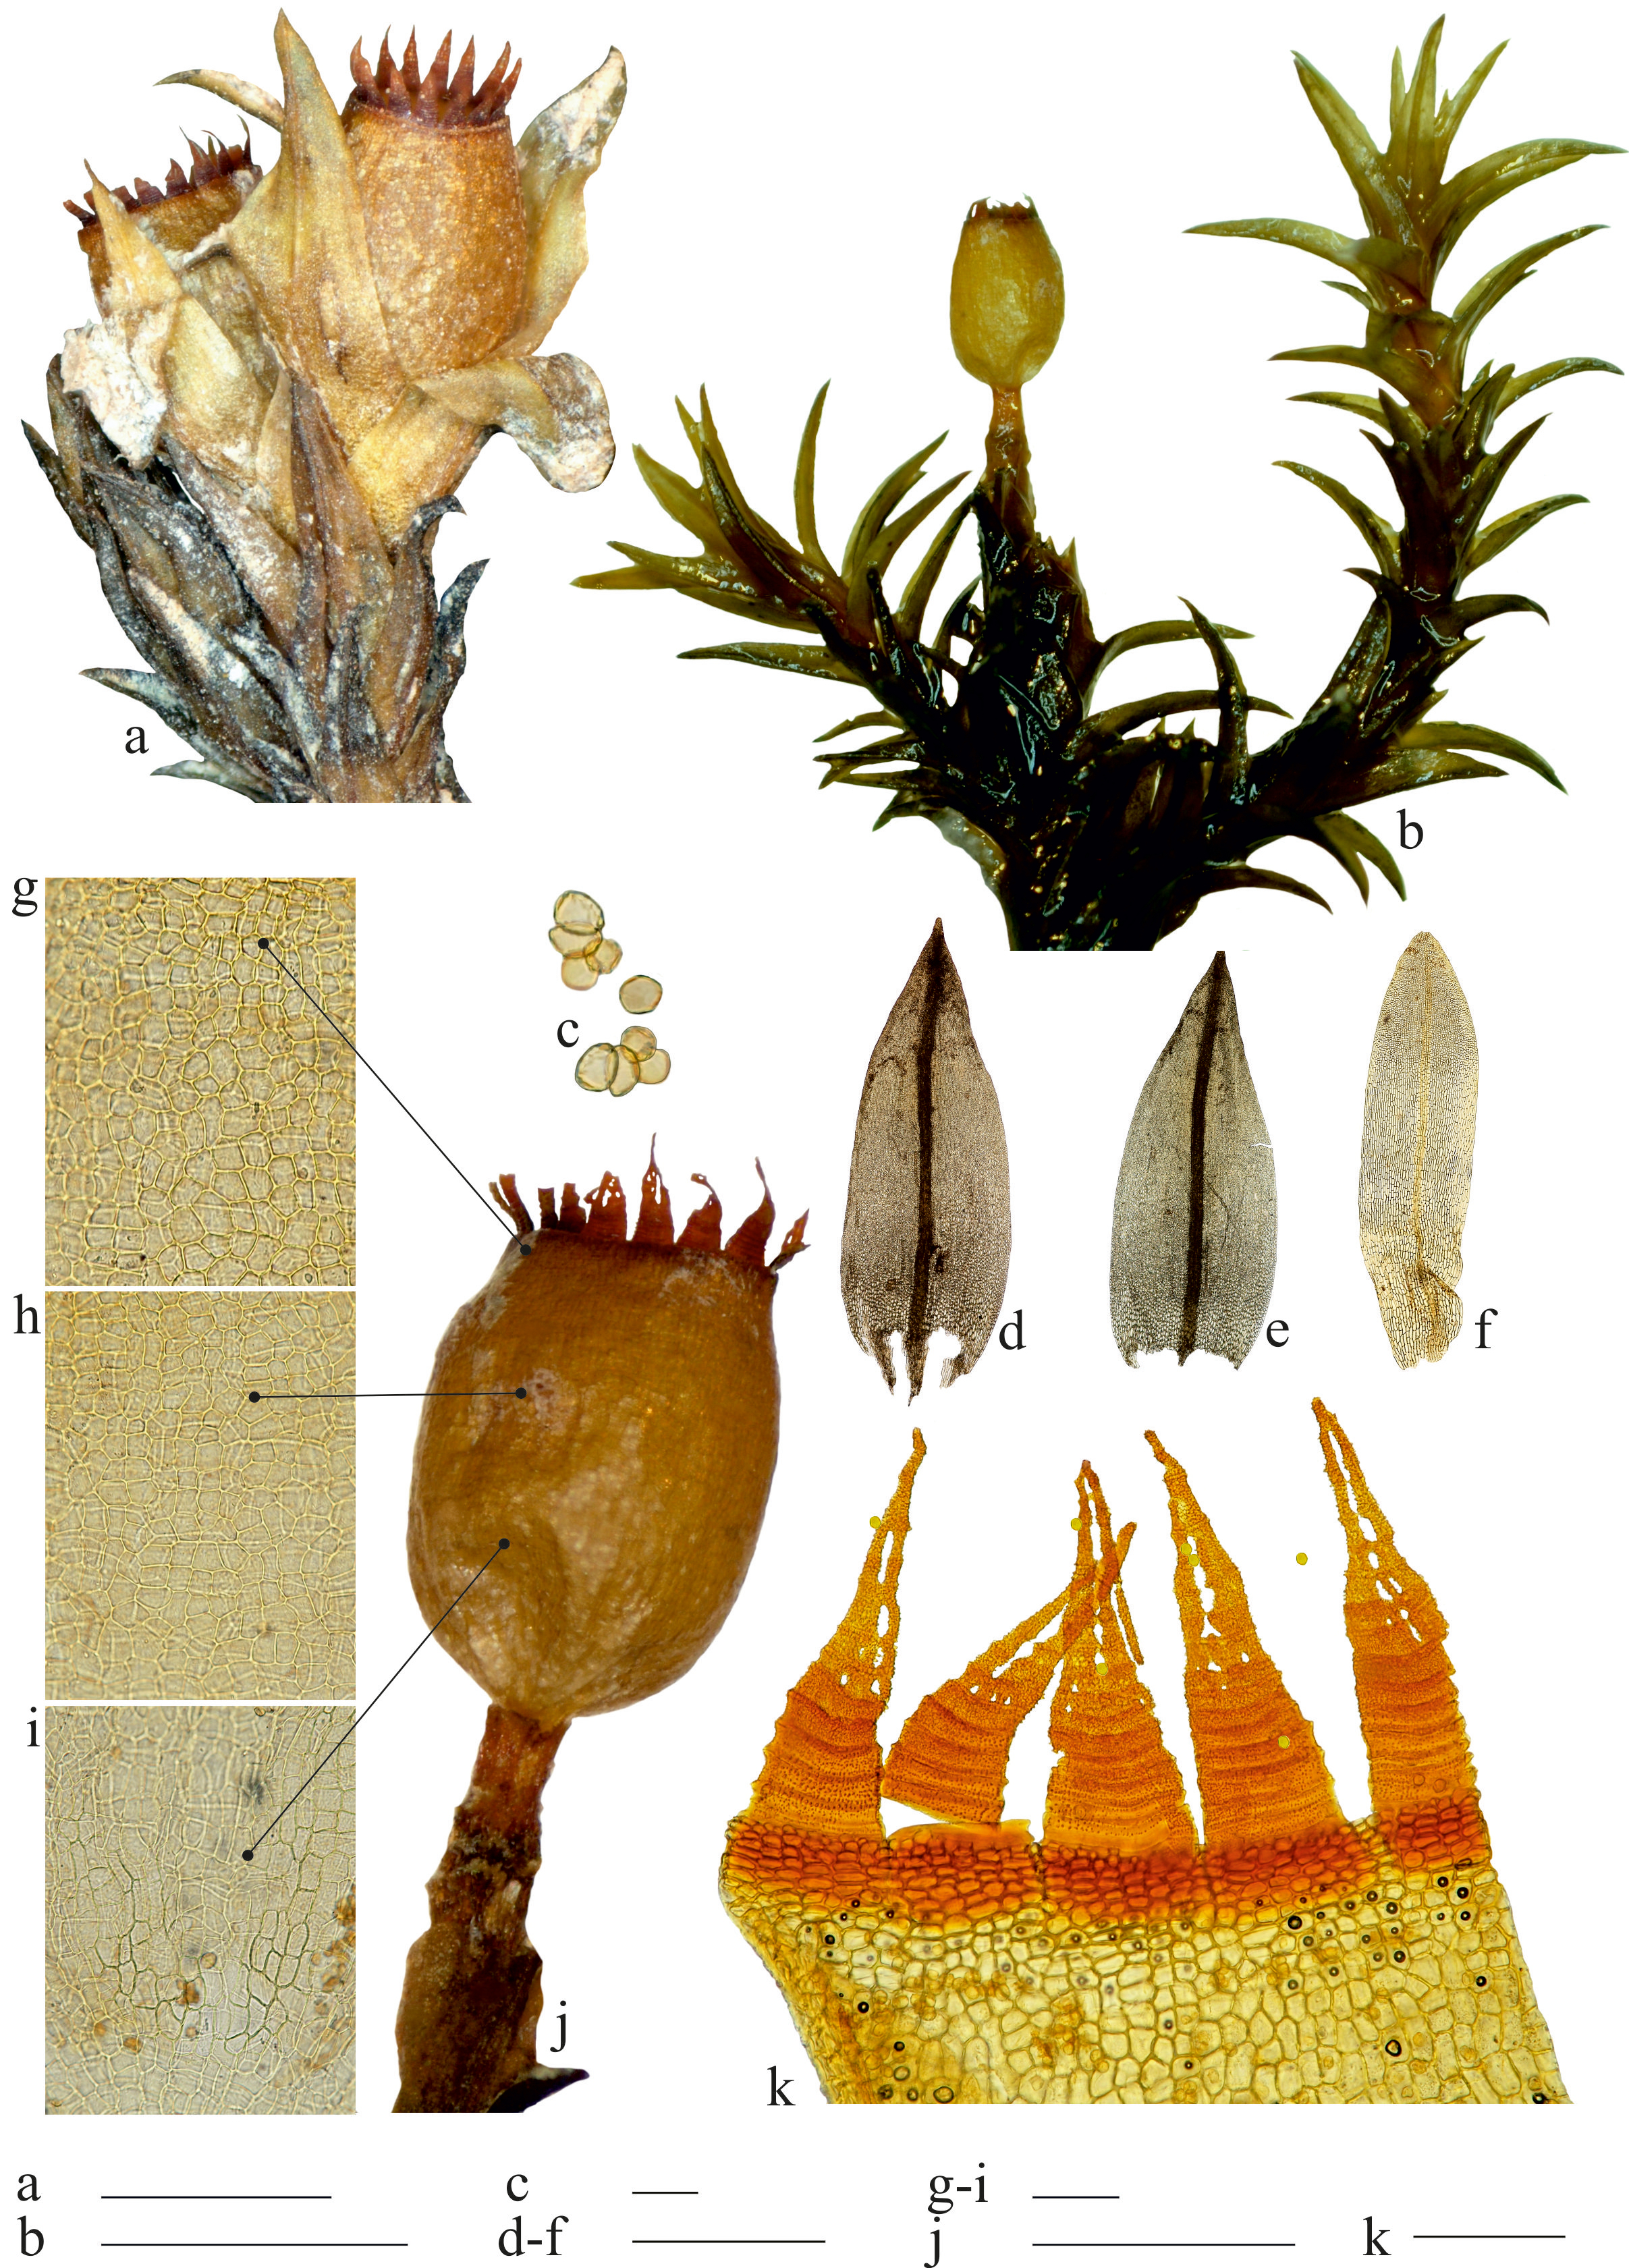
Figure 3
SEM micrographs of the peristome teeth and spores of Schistidium deguchianum taken from the specimen from Jauja Province in Peru: (a, c) inner surface of the peristome teeth, (b, d) outer surface of the peristome teeth, (e-g) spores. All data were obtained from MO 5143304. Scale bars: (a, c) 50 μm; (e-g) 5 μm.
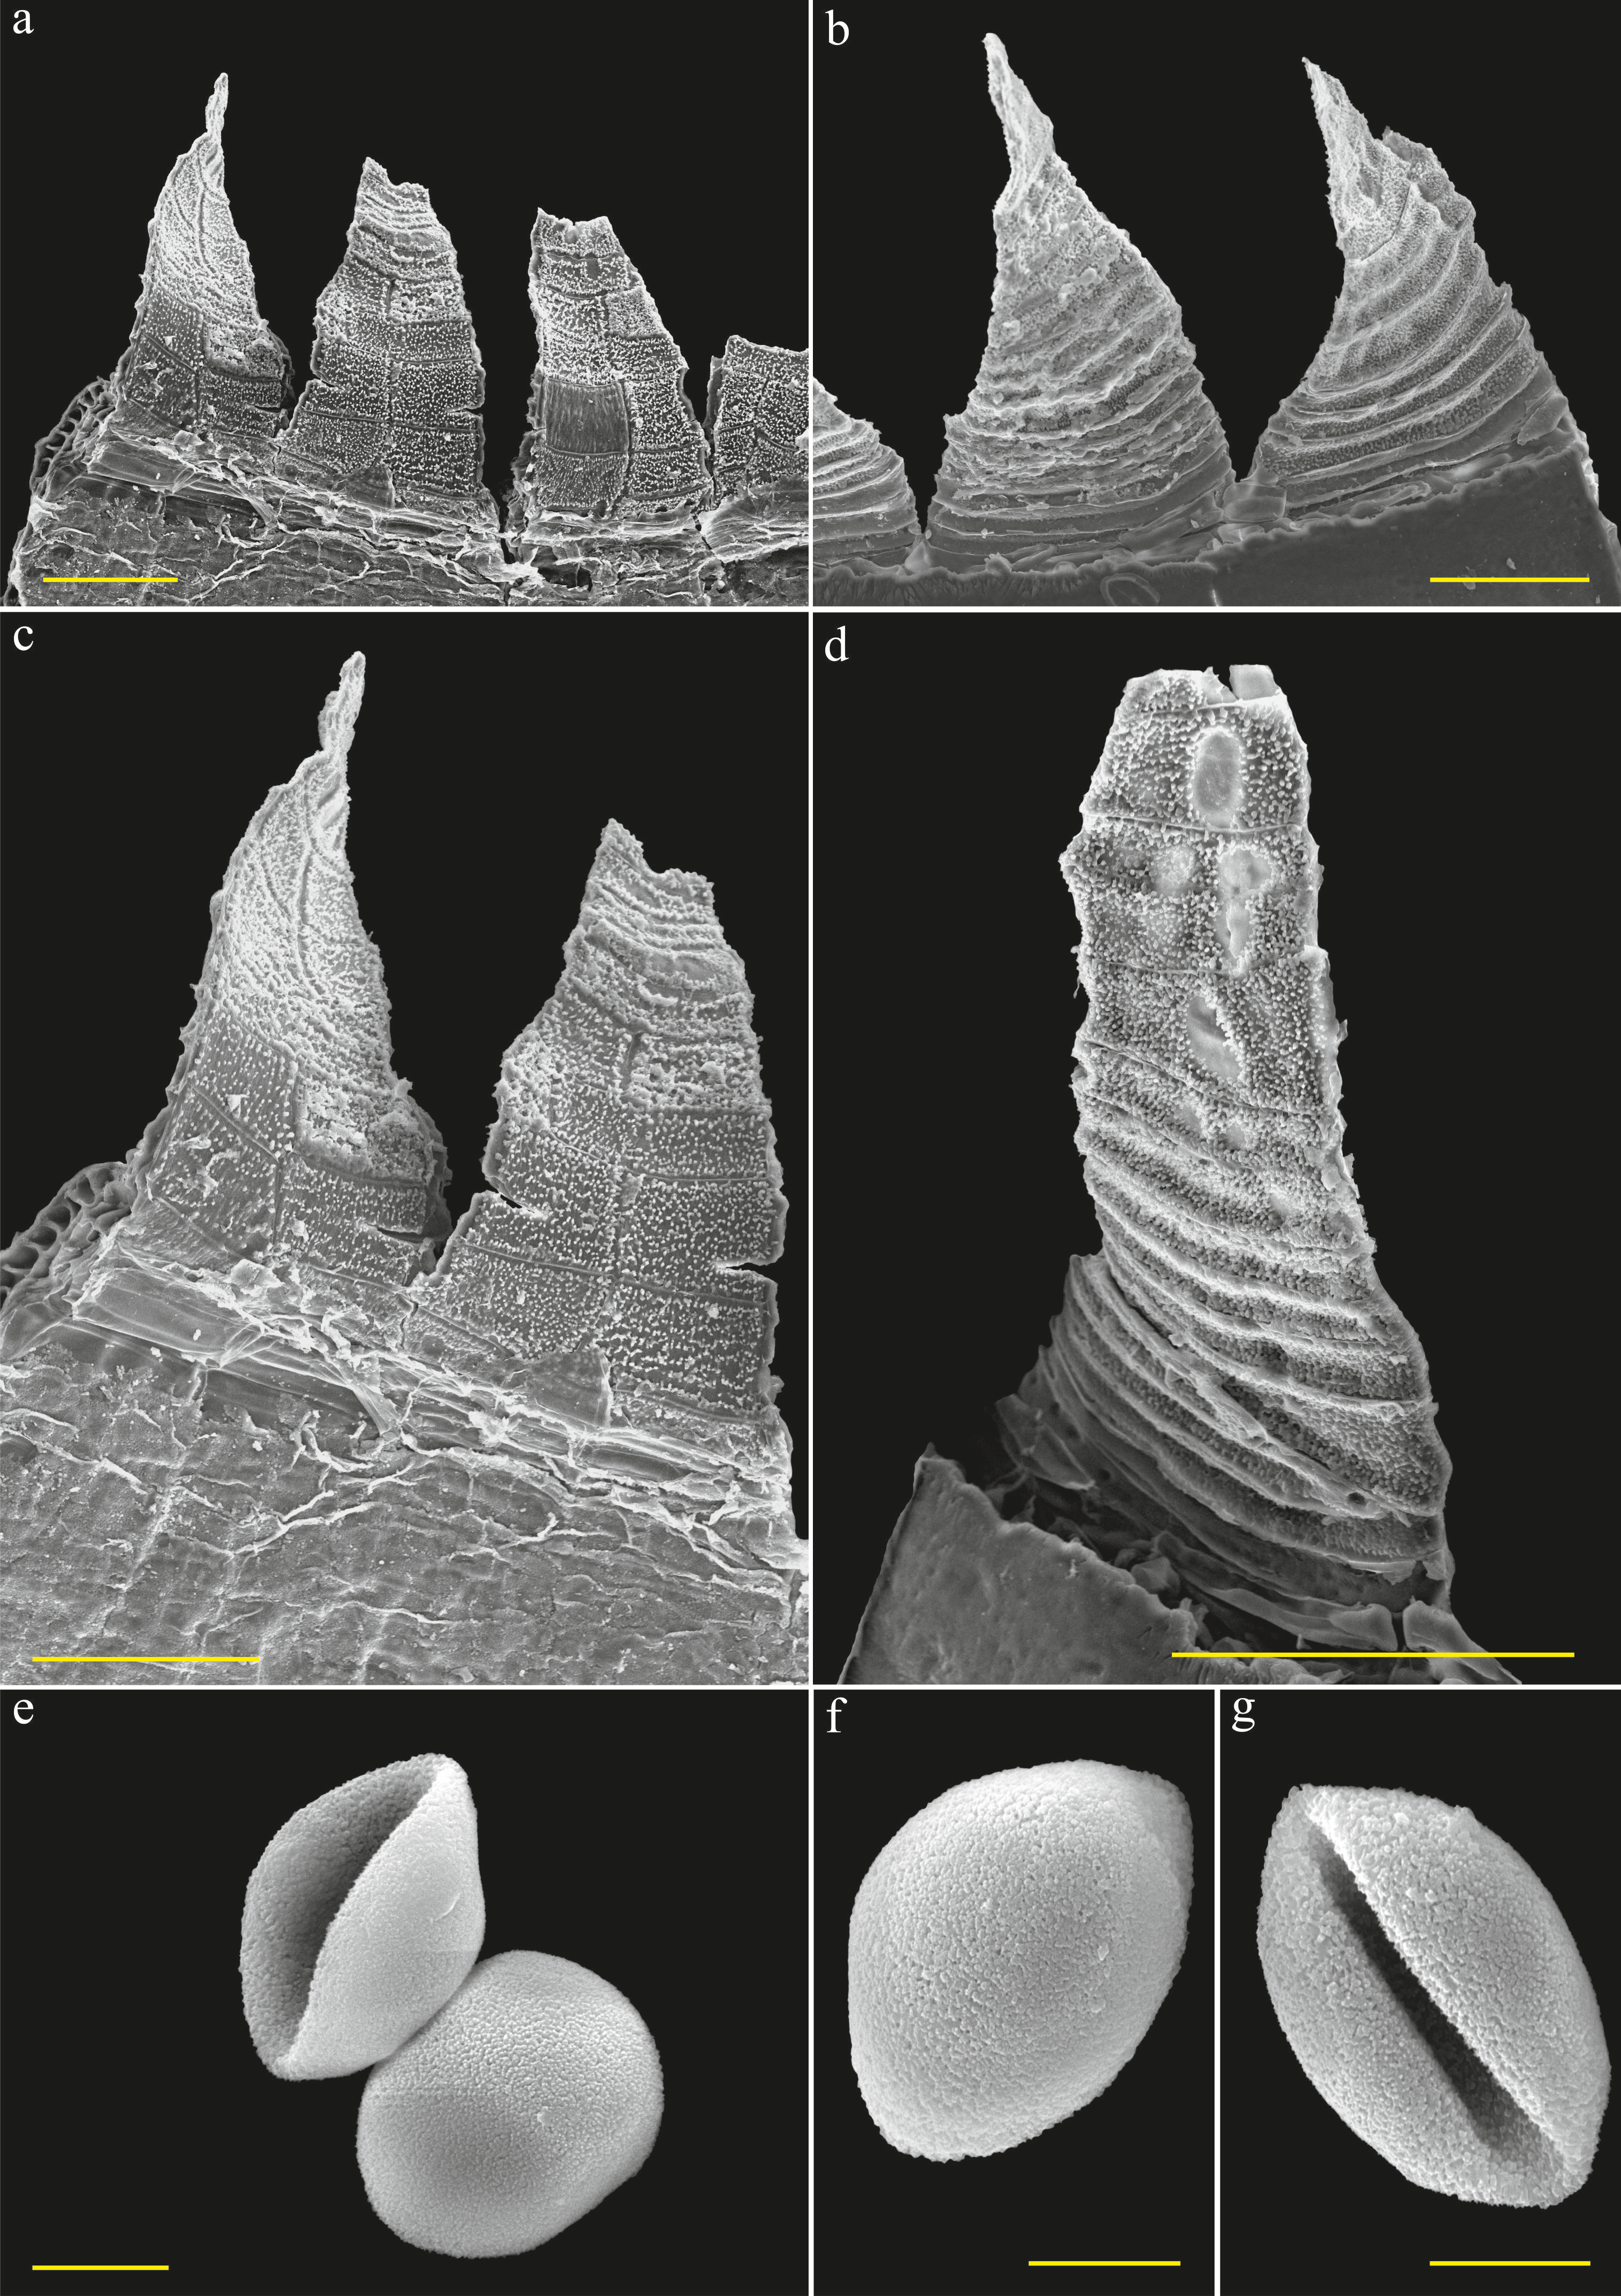
The plants are gonioautoicous. The perichaetial leaves are erect, oblong to ovate-lanceolate, 2.2–2.7 mm long and 0.9–1.0 mm wide, gradually acuminate, with an acute, epilose apex. The laminal cells are unistratose throughout, with some bistratose strands in the leaf apex. In the innermost bracts, the laminal cells are small, isodiametric, and somewhat irregular in shape at the apex, becoming short-rectangular toward the mid-leaf and rectangular, thin-walled, transparent, and hyaline, but not lax in the proximal half. The leaf margins are plane, entire or slightly uneven near the apex, and unistratose or partially bistratose in a single cell row. The costa is percurrent, weak, and concolorous with the laminal cells, measuring 40–50 μm in width in the lower half, becoming prominent, yellow, and sharply differentiated from the laminal cells in the distal portion. Sporophytes are abundant and shallowly immersed. The seta is stout, thick, straight, and 0.3–0.35 mm long. The capsules are systylious, pale brown, and leptodermous, ranging from obloid to short cylindrical, 1.0–1.4 mm long and 0.7–0.8 mm wide, with a length-to-width ratio of 1.4–1.7(–1.9) when fresh, and are abruptly contracted into the seta. The exothecial cells are thin-walled and variable in size and shape, mostly short, quadrate, rhombic, or irregular, and occasionally transversely rectangular to oblong in the mid-urn, measuring 10–24 × 15–35 μm. At the base of the urn, the cells are predominantly short-rectangular, becoming smaller, rounded, and elliptical to oblate in 4–5 rows near the urn mouth, where they form an intensely orange-brown band. Stomata are absent. The peristome is single and consists of 16 teeth that are erect when dry; orange, lanceolate, and mostly asymmetric with uneven margins, 300–350 μm long, and 80–100 μm wide at the base, gradually tapering to an acute or obtuse apex. In the distal half, the teeth are variously perforated or narrowly fissured, distinctly cross-barred, and densely papillose on both the outer and inner surfaces, bearing short, broad, warty papillae. The columella is permanently attached to the operculum and is long and narrow. The operculum is conic-convex with a straight rostrum and measures 0.5–0.7 mm in length. The spores are subspherical, measuring 10–12 μm in diameter, and finely papillose. The calyptra is small, mitriform or cucullate, split into 4–5 lobes at the base, covering only the rostrum, and not reaching the rim of the capsule.
Specimen examined: PERU. Junin Region, Jauja Province: Río Pachayo near Conchayllo between La Oroya and Jauja, alt. 3650 m a.s.l., lat. 11°50'S, long. 75°45'W, on a boulder in stream, July 10, 1977, leg. P. & E. Hegewald 9277 (MO 5143304).
. Taxonomic and phytogeographical notes on Schistidium deguchianum
Although the Peruvian specimen was originally identified as Schistidium cinclidodonteum, S. deguchianum differs from it in numerous respects. The leaves of S. cinclidodonteum are typically strongly falcate-secund, with entire margins throughout, and are narrowly linear-lanceolate, gradually tapering into a long subulate acumen that is acute or blunt at the apex. In transverse sections, they are mainly bistratose in the uppermost part of the subula, becoming unistratose below down to the base, only occasionally with irregular bistratose streaks. The stem lacks a central strand, and the costa is relatively broad, measuring 100–140 μm at the base. The capsule is obloid to short cylindrical, 1.3–2.0 mm long and 0.8–1.0 mm wide, with a length-to-width ratio of 1.6–2.0.
In contrast, the leaves of Schistidium deguchianum are usually straight to slightly curved, ovate-lanceolate to lanceolate, and gradually acuminate to a short acute apex, with bluntly serrulate or sinuate margins. They are perfectly bistratose in the upper half, with unistratose patches occurring only near the costa in the basal part, and 3–4-stratose patches at the margins in the distal part, forming fleshy, multiseriate, somewhat bulging marginal borders that extend to the leaf-base. Additionally, the stem possesses a well-developed central strand, and the costa is weaker and narrower, 80–90 μm wide near the base. The capsule is similar in shape but smaller, measuring 1.0–1.4 mm in length and 0.7–0.8 mm in width, with a length-to-width ratio of 1.4–1.7.
The second species with which Schistidium deguchianum may be confused is S. falcatum, a Holantarctic species occurring on subantarctic islands, extending very rarely to the maritime Antarctic, and scattered in the Andes from Tierra del Fuego through Patagonia to Bolivia. This species closely resembles S. cinclidodonteum in leaf shape and size, but differs in having a slightly narrower costa, 85–120 μm wide at the leaf base, and leaf cells that are unistratose in the lower and middle parts of the leaf, becoming only irregularly 1–2-layered toward the apex. Furthermore, it possesses a smaller capsule, subglobose to shortly obloid, 0.8–1.3 mm long and 0.7–1.0 mm wide, with a length-to-width ratio of 1.1–1.3, and larger spores, 20–28 μm in diameter. In addition, S. falcatum differs from both species in its exothecial cells, which are firm and sturdy with slightly thickened walls, whereas S. cinclidodonteum and S. deguchianum have consistently thin-walled exothecial cells.
Although most species within the genus Schistidium are xerophytic mosses that grow on dry, exposed, and insolated rocks, a relatively large group of rheophytic species is an important component of riparian habitats. These species inhabit rocks and boulders in streams and waterfalls with fast-flowing water and exhibit a range of morphological and anatomical characteristics that are adapted to such environments. One notable feature is the multilayered structure of the leaf lamina, often accompanied by salient, frequently spurred costae, and prominently thickened, fleshy leaf margins. These traits are generally regarded as structural adaptations to life in fast-flowing water and are found in numerous species across different, often unrelated genera and families (Bednarek-Ochyra et al., 1996; Bednarek-Ochyra & Ochyra, 2012b; Ochyra, 1985a, 1985b, 1986, 1987b; Ochyra & Matteri, 2001; Ochyra & van Rooy, 2013; Ochyra & Vanderpoorten, 1999). The largest group, comprising 13 species, is assigned to subg. Canalicularia Ochyra is characterized by concave leaves with plane and erect margins, whereas six species are placed in subg. Apocarpa (Vilh.) Ochyra (Blom et al., 2011; Ochyra, 2003; Ochyra & Bednarek-Ochyra, 2015). However, their precise phylogenetic relationships have not been investigated.
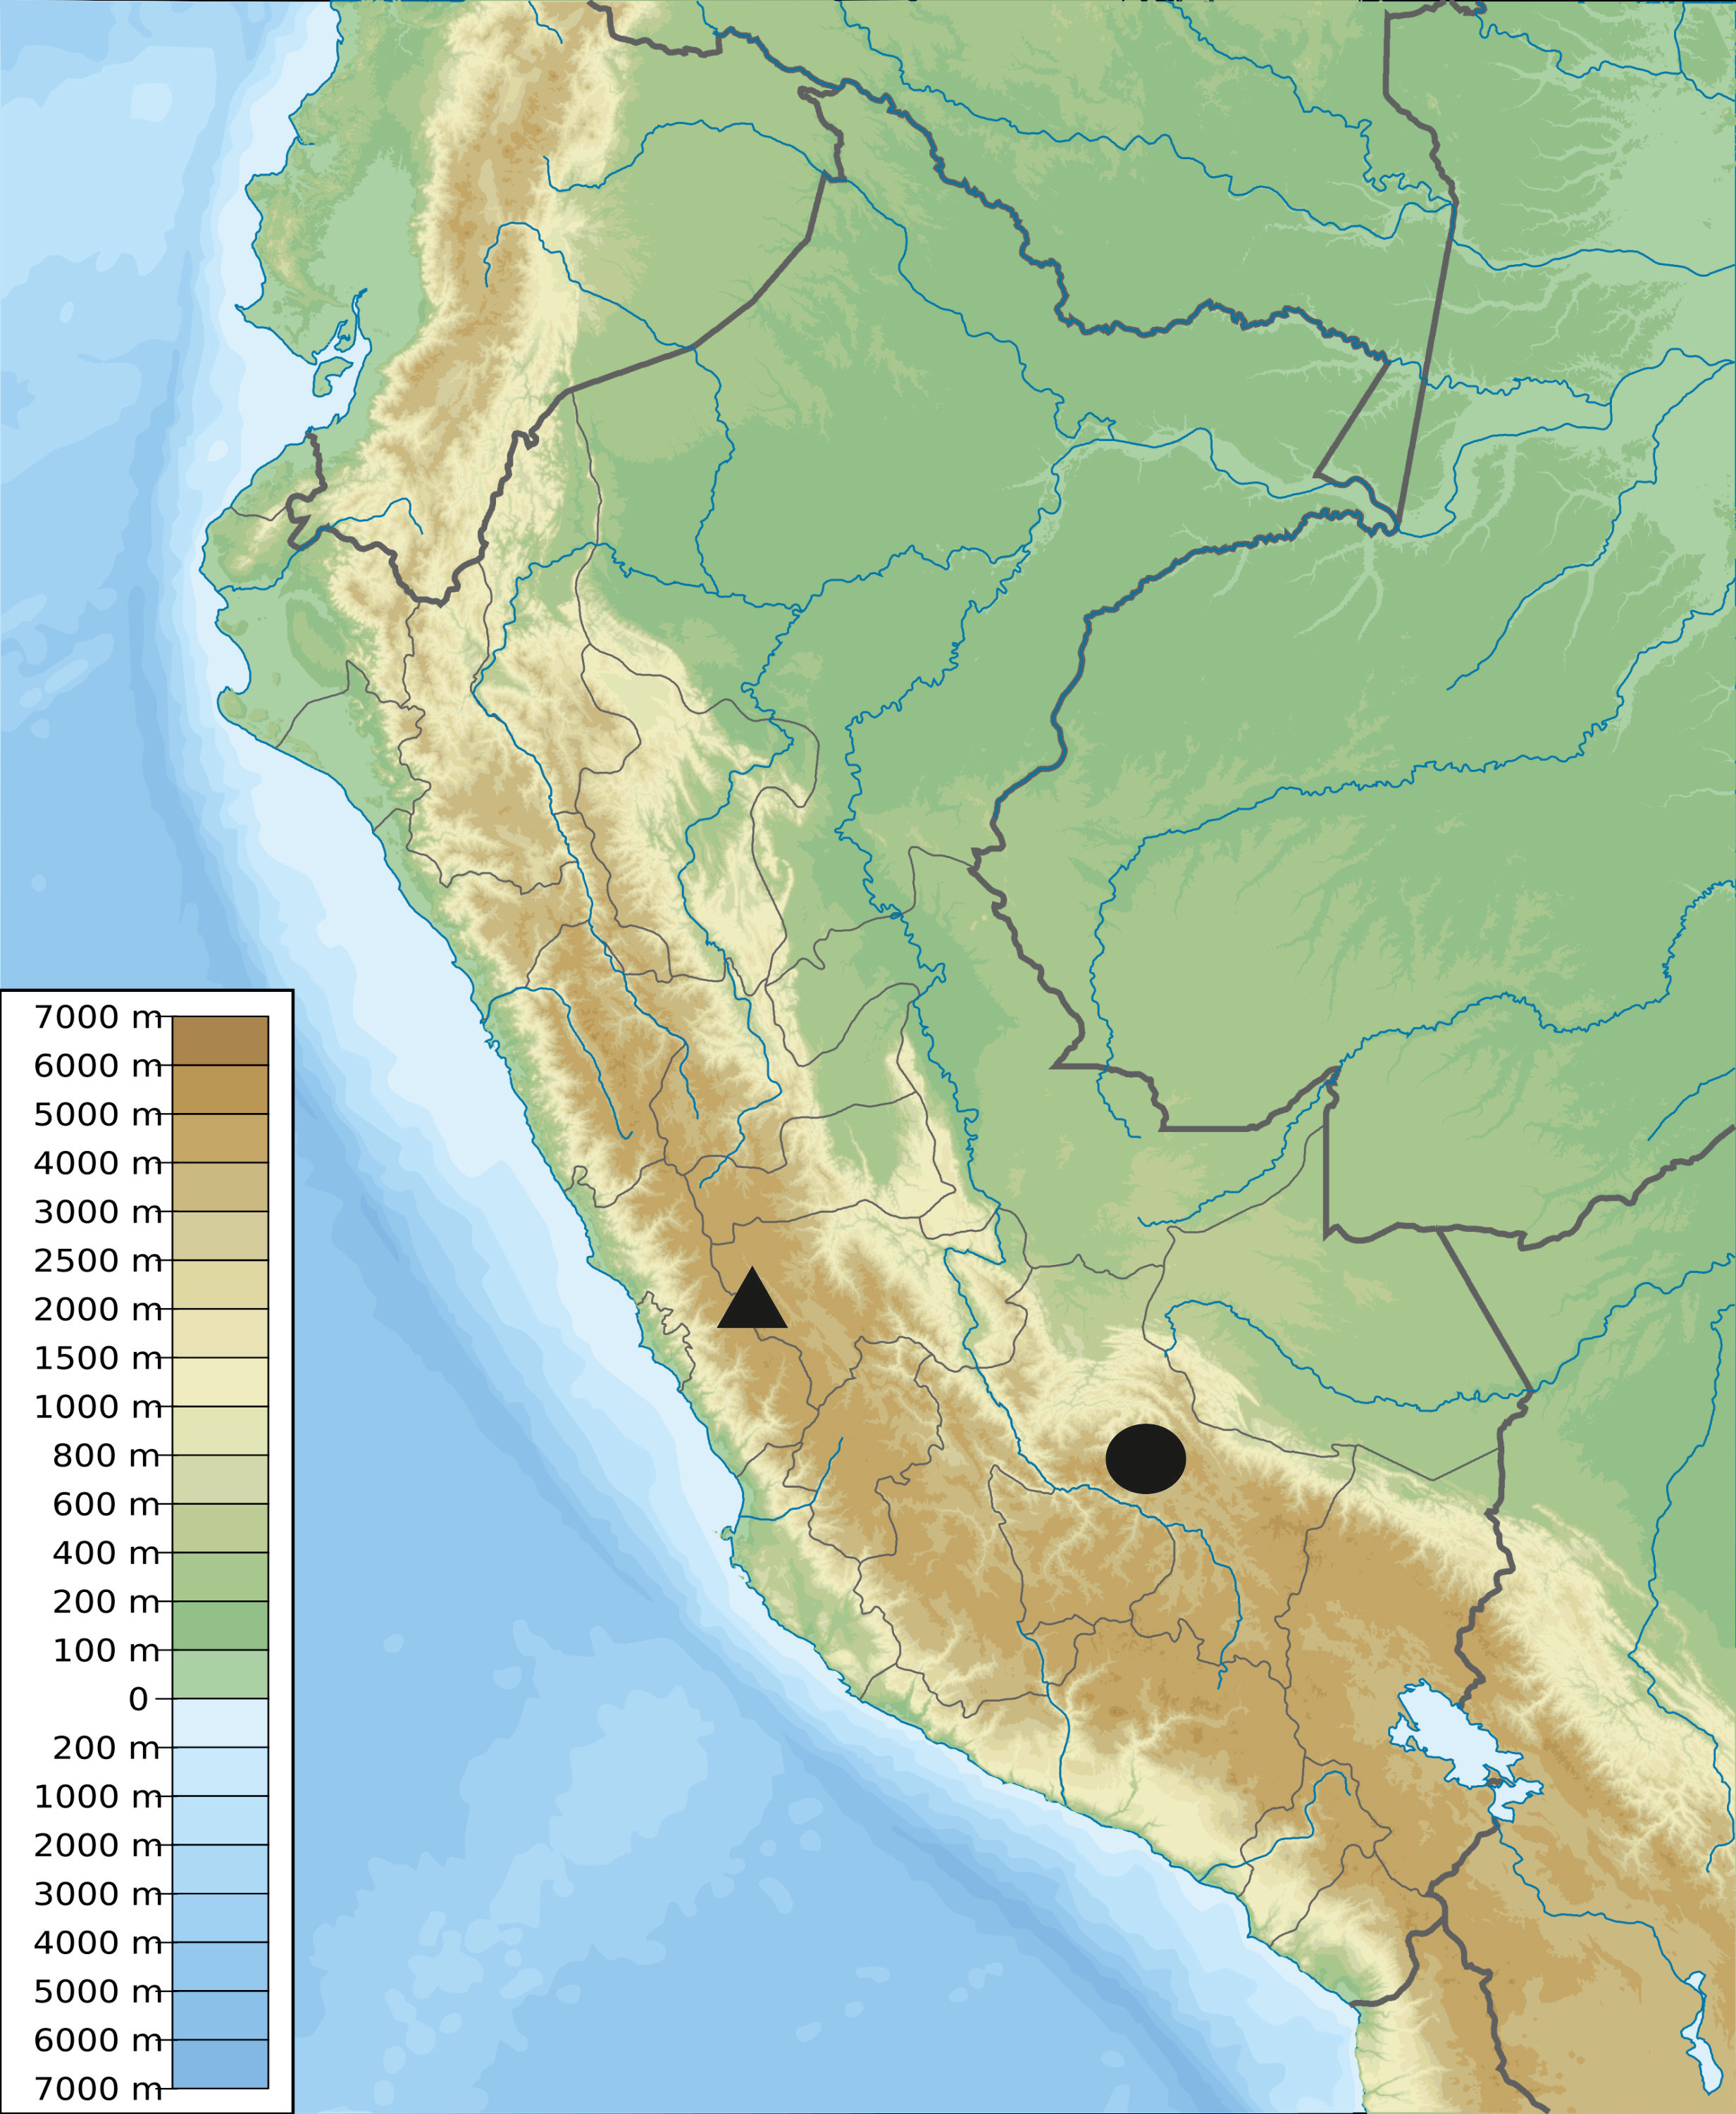
To date, Schistidium deguchianum has been documented only from a single collection made at an elevation of 3000 m a.s.l. in the Eastern Cordillera, Urubamba Province, Cusco Region, Peru (Figure 4). The newly reported locality lies at 3650 m a.s.l. in the Central Cordillera, within the Jauja Province, Junín Region, approximately 400 km in a straight line from the locus classicus. Unfortunately, no additional habitat data are available for this site, apart from the fact that the moss was collected on boulders in a stream, which is a typical habitat for rheophytic mosses.
Figure 4
Distribution map of Schistidium deguchianum in Peru. Black dot: locus classicus; triangle: new locality.
Schistidium deguchianum is the fourth species of this genus recorded in Peru. The first was S. streptophyllum (Sull.) Herzog (Sullivant, 1859), which has also been reported from Bolivia (Bremer, 1980b; Herzog, 1916). The second, S. rivulariopsis (R.S. Williams) Ochyra was described from the same locality as S. deguchianum (Williams, 1916), with which it occurred in a mixed stand, as noted by Deguchi (1987). This author initially regarded this taxon as conspecific with S. rivulare (Brid.) Podp.; however, it was subsequently recognized as a distinct species (Ochyra & Bednarek-Ochyra, 2011). Additional records of S. rivulariopsis in South America have been reported from Colombia (Ellis et al., 2015b) and Kenya in East Africa (Ellis et al., 2016b). This species has also been reported from Ecuador (Bartram, 1955), but the voucher specimens represent a different species whose final identity still needs examination (Ochyra & Bednarek-Ochyra, 2011). It is worth noting that Churchill et al. (2000) considered S. rivulariopsis to be conspecific with the Holarctic S. platyphyllum (Mitt.) H. Perss., but this species has larger and granulose spores, which immediately separate these species. Accordingly, S. platyphyllum has been excluded from the moss flora of South America.
Finally, the third species currently known from Peru, and so far, recorded from a single locality, is S. yaulense (Broth.) Ochyra & J. Muñoz. This species was originally described as Grimmia yaulensis Broth. (Brotherus, 1920). This requires critical re-examination and lectotypification, as the type specimen contains material referable to more than one species.
. Diversity of Schistidium in South America
Due to their distinctive morphology, particularly that of the sporophytes, mosses of the genus Schistidium are readily distinguishable from other moss genera and have traditionally been unambiguously assigned to Schistidium within the family Grimmiaceae. Over the more than 183 years since the first specimens were collected (1842–2025), 36 species and three unnamed varieties have been reported from mainland South America, including the Falkland Islands (Table 1). South Georgia, a large subantarctic island in the Scotia Arc, was excluded from the present study because, from a botanical perspective, it belongs to a different southern polar biome and exhibits closer affinities to the flora and vegetation of the maritime Antarctic.
Table 1
A chronological list of species and varieties of the genus Schistidium described and recorded in South America between 1847 and 2025. Names in capital letters refer to currently accepted taxa; names in bold indicate taxa described from South American material; names in both capital letters and bold denote taxa described from South America that are accepted in modern taxonomy. Names in capital letters but not in bold indicate currently accepted species that were originally described outside South America and are reported here for the first time from this continent. Accepted species presented in regular type in the column “Current status” refer to secondary records of the species. Names in lowercase but bold indicate species that have not been re-examined since their original descriptions but are likely to be accepted as distinct species.
| No. | Taxon | Country or region | Publication | Current status | First synonymisation or change of the taxonomic status |
|---|---|---|---|---|---|
| 1. | Grimmia maritima Sm. ex R. Scott | Chile | Wilson & Hooker (1847) | Schistidium Bruch & Schimp. sp. | Present paper |
| 2. | Grimmia apocarpa Hedw. var. 1 | East Falkland | Wilson & Hooker (1847) | Schistidium Bruch & Schimp. sp. | Present paper |
| 3. | Grimmia apocarpa Hedw. var. 4 | Chile | Wilson & Hooker (1847) | SCHISTIDIUM AMBLYOPHYLLUM (Müll.Hal.) Ochyra & Hertel | Müller (1849) |
| 4. | Grimmia amblyophylla Müll.Hal. | Chile | Müller (1849) | Schistidium amblyophyllum (Müll.Hal.) Ochyra & Hertel | Ochyra & Hertel (1990) |
| 5. | Grimmia apocarpa Hedw. var. α - Foliis muticis (Schimp., in litt.) | Chile | Montagne (1850) | Schistidium Bruch & Schimp. sp. | Present paper |
| 6. | Grimmia streptophylla Sull. | Peru | Sullivant (1859) | SCHISTIDIUM STREPTOPHYLLUM (Sull.) Herzog | Herzog (1916) |
| 7. | Grimmia saxatilis Mitt. | Ecuador | Mitten (1869) | SCHISTIDIUM SAXATILE (Mitt.) Ochyra | Ochyra (1998b) |
| 8. | Grimmia andina Mitt. | Ecuador | Mitten (1869) | SCHISTIDIUM ANDINUM (Mitt.) Herzog | Herzog (1916) |
| 9. | Grimmia angustifolia Mitt. | Ecuador | Mitten (1869) | SCHISTIDIUM ANGUSTIFOLIUM (Mitt.) Herzog | Herzog (1916) |
| 10. | Guembelia lorentziana Müll.Hal. | Argentina | Müller (1882) | Schistidium andinum (Mitt.) Herzog | Ochyra et al. (2008b) |
| 11. | Guembelia praemorsa Müll.Hal. | Argentina | Müller (1882) | SCHISTIDIUM PRAEMORSUM (Müll.Hal.) Herzog | Herzog (1916) |
| 12. | Grimmia fallax Dusén | Argentina | Dusén (1903) | Schistidium andinum (Mitt.) Herzog | Ochyra et al. (2008b) |
| 13. | Grimmia fasciculata Dusén, hom. illeg. | Chile | Dusén (1905) | SCHISTIDIUM FALCATUM (Hook.f. & Wilson) B. Bremer | Bremer (1980b) |
| 14. | Grimmia apocarpa Hedw. | Argentina, Chile, East Falkland | Cardot (1908) | Schistidium apocarpum (Hedw.) Bruch & Schimp. – excluded | Present paper |
| 15. | Grimmia occulta Müll.Hal. | Argentina, Chile | Cardot (1908) | Schistidium andinum (Mitt.) Herzog | Ochyra et al. (2008b) |
| 16. | Grimmia abscondita Cardot | Argentina | Cardot (1908) | Schistidium praemorsum (Müll.Hal.) Herzog | Ochyra et al. (2008b) |
| 17. | Grimmia calycina Herzog | Bolivia | Herzog (1910) | Schistidium calycinum (Herzog) Ochyra | Ochyra (1998b) |
| 18. | Schistidium subpraemorsum Broth. | Bolivia | Herzog (1916) | Schistidium angustifolium (Mitt.) Herzog | Present paper |
| 19. | Schistidium chocayae Herzog | Bolivia | Herzog (1916) | – – – | |
| 20. | SCHISTIDIUM MALACOPHYLLUM Herzog | Bolivia | Herzog (1916) | – – – | |
| 21. | Schistidium tunariense Herzog | Bolivia | Herzog (1916) | Schistidium angustifolium (Mitt.) Herzog | Bremer (1980b) |
| 22. | Schistidium fontanum Herzog | Bolivia | Herzog (1916) | Schistidium falcatum (Hook.f. & Wilson) B. Bremer | Bremer (1980b) |
| 23. | Grimmia olivacea Herzog | Bolivia | Herzog (1916) | Schistidium olivaceum (Herzog) Ochyra & J. Muñoz | Ochyra & Muñoz (2000) |
| 24. | Grimmia squamatula Herzog | Bolivia | Herzog (1916) | Schistidium squamatulum (Herzog) Ochyra & J. Muñoz | Ochyra & Muñoz (2000) |
| 25. | Grimmia rivulariopsis R.S. Williams | Peru | Williams (1916) | SCHISTIDIUM RIVULARIOPSIS (R.S. Williams) Ochyra | Ochyra (1998b) |
| 26. | Grimmia yaulensis Broth. | Peru | Brotherus (1920) | Schistidium yaulense (Broth.) Ochyra & J. Muñoz | Ochyra & Muñoz (2000) |
| 27. | Grimmia perplexa Thér. | Chile | Thériot (1923) | Schistidium perplexum (Thér.) Ochyra | Ochyra (1998b) |
| 28. | Grimmia conferta Funck | Argentina, East Falkland | Cardot & Brotherus (1923) | Schistidium confertum (Funck) Bruch & Schimp. – excluded | Present paper |
| 29. | Grimmia alpicola Hedw., nom. rejic. | Argentina | Cardot & Brotherus (1923) | Schistidium agassizii Sull. & Lesq. – excluded | Present paper |
| 30. | Grimmia alpicola var. rivularis (Brid.) Wahlenb. | Argentina | Cardot & Brotherus (1923) | SCHISTIDIUM RIVULARE (Brid.) Podp. | – |
| 31. | Grimmia celata Cardot | Argentina | Cardot & Brotherus (1923) | SCHISTIDIUM CUPULARE (Müll.Hal.) Ochyra | Ochyra (2004b) |
| 32. | Grimmia macrotyla Cardot & Broth. | Argentina | Cardot & Brotherus (1923) | Schistidium macrotylum (Cardot & Broth.) Ochyra | Ochyra (1998b) |
| 33. | Grimmia hyalinocuspidata Cardot & Broth. | Chile | Cardot & Brotherus (1923) | Schistidium angustifolium (Mitt.) Herzog | Present paper |
| 34. | Grimmia chubutensis Cardot & Broth. | Argentina | Cardot & Brotherus (1923) | Schistidium praemorsum (Müll.Hal.) Herzog | Ochyra et al. (2008b) |
| 35. | Grimmia syntrichiacea Müll.Hal. | Argentina | Cardot & Brotherus (1923) | Schistidium andinum (Mitt.) Herzog | Ochyra et al. (2008b) |
| 36. | Schistidium chrysoblastum Herzog | Bolivia | Herzog (1934) | Schistidium angustifolium (Mitt.) Herzog | Bremer (1980b) |
| 37. | Grimmia donatii Herzog & Thér. | Chile | Herzog (1937) | Schistidium angustifolium (Mitt.) Herzog | Present paper |
| 38. | Grimmia scabripes E.B. Bartram | Chile | Bartram (1946) | SCHISTIDIUM SCABRIPES (E.B. Bartram) Deguchi | Deguchi (1984) |
| 39. | Schistidium platyphyllum (Mitt.) H. Perss. | Peru, Ecuador | Churchill et. al. (2000) | Excluded | Present paper |
| 40. | SCHISTIDIUM DEGUCHIANUM Ochyra & Bedn.-Ochyra | Peru | Ochyra & Bednarek-Ochyra (2011) |
Most of these taxa were originally reported under the generic name Grimmia, with two species assigned to Guembelia Hampe and only seven described or recorded under the name Schistidium. Owing to the historically underdeveloped taxonomy of this genus, which has only recently undergone substantial revision in Europe, it remains difficult to draw detailed conclusions or to provide a comprehensive synthesis. For a long time, the genus was treated according to an overly broad and unrealistic taxonomic concept, in which nearly all specimens exhibiting the characteristics of Schistidium were subsumed under a single species, S. apocarpum. Consequently, this taxon has become an ill-defined assemblage encompassing a wide range of phenotypes, many of which represent distinct species. A clear illustration of this problem is the assignment of 24 specimens collected from numerous localities in Peru to S. apocarpum, including specimen No. 9277, which is described in this paper as S. deguchianum (Hegewald & Hegewald, 1985).
Accordingly, this study aimed to summarize the current state of knowledge of the genus Schistidium in South America and provide a foundation for its future revision. Attention is drawn to morphological characters of high diagnostic value that are now widely recognized in species delimitation but were largely overlooked in earlier studies. The application of these characters has led to the continued description of new species in Europe (Blom et al., 2016, 2025; Guerra et al., 2019, 2020; Kiebacher et al., 2021, 2024), a region that is nevertheless among the most intensively studied in bryology.
Of the 37 species of Schistidium reported from South America, five must be excluded from the bryoflora: S. maritimum, S. apocarpum, S. confertum, S. agassizii, and S. platyphyllum. These are Holarctic taxa, and the examined voucher specimens on which these reports are based almost certainly represent different species; however, their precise identity cannot be determined at this stage of research. Similarly, the status of the three unnamed varieties requires clarification. Grimmia apocarpa var. 4, originating from Hermite Island, was described by Müller (1849) as a separate species and is now accepted as S. amblyophyllum. The other two specimens also appear to constitute separate species. To date, 27 species have been described from South America. Of these, ten are currently accepted, ten are regarded as conspecific with other species, and seven have not been taxonomically assessed since their original descriptions. Nevertheless, there are strong indications that future taxonomic revisions may support their recognition as distinct species in the future. Only three species currently accepted in the South American bryoflora were originally described from outside the continent: S. falcatum and S. cupulare from the subantarctic Îles Kerguelen and S. rivulare from Europe. Ongoing field studies across various regions of South America continue to yield new specimens of Schistidium, some of which may represent previously undescribed species in the future. They are occasionally found in unusual habitats such as tree bark. This evidence strongly suggests that the diversity of the genus remains underestimated, rendering any conclusions regarding species richness and distribution across regions or countries premature.
There is a clear analogy here with the neighboring Antarctic, where the diversity of the genus Schistidium has increased rapidly because of comprehensive studies of the continent’s moss flora, combined with parallel fieldwork and taxonomic revision of all available material. Five new species have been described from this region (Ochyra, 1987a, 1998a, 2003, 2004c; Ochyra et al., 2003), and several species previously known only from South America and South Georgia, namely S. andinum, S. praemorsum, S. cupulare, S. falcatum, and S. urnulaceum, have also been recorded there (Ochyra & Bell, 1984; Ochyra, 1990; Ochyra et al., 2008b).
A correction is required regarding the occurrence of Schistidium amblyophyllum in Antarctica. The Antarctic material belongs to S. angustifolium, a species that was previously erroneously considered conspecific with S. amblyophyllum. The two species share very similar leaf areolation, which led to this taxonomic interpretation. However, examination of many S. amblyophyllum specimens from Tierra del Fuego has convincingly demonstrated that they differ markedly in the shape of the perichaetial leaves: in S. amblyophyllum, these are broadly rounded at the apex, whereas in S. angustifolium, they are pointed and terminate in hyaline hair-like tips.
. Chorotypes of South American species of Schistidium
All accepted South American Schistidium species represent several chorotypes in this study. Notably, only one bipolar species, S. rivulare, has been recorded in the moss flora of South America, whereas all other species are restricted to the Southern Hemisphere. The largest group, comprising 12 species, consists of endemics, five of which are generally accepted: S. streptocarpum, S. saxatile, S. scabripes, S. deguchianum, and S. malacophyllum. The latter species was recently considered conspecific with S. rivulare (Suárez et al., 2018); however, this interpretation is difficult to accept, as S. malacophyllum is characterized by small, nearly smooth spores and strongly concave leaves with entire, flat, and erect margins. The remaining seven endemic taxa are known only from type specimens and have not yet undergone a thorough taxonomic evaluation. These species are Schistidium calycinum, S. chocayae, S. olivaceum, S. squamatulum, S. yaulense, S. macrotyla, and S. perplexum.
The next chorotype is represented by amphiatlantic southern cool-temperate species that occur, on the one hand, in southern South America and on South Georgia and, on the other, on islands of the Kerguelen Province in the South Indian Ocean. This distribution pattern is relatively well represented among mosses and liverworts (Ochyra, 1987c, 1989b, 2010; Ochyra & Váňa, 1989; Bednarek-Ochyra & Ochyra, 1998, 2013; Ochyra & Lewis Smith, 1998; Ochyra & Zander, 2002; Ochyra et al., 2002a; Ochyra & Singh, 2008; Li et al., 2009; Blockeel et al., 2009a, 2009b; Ellis et al., 2012b, 2012c, 2013, 2015a, 2015c, 2017, 2019; Ochyra & Bednarek-Ochyra, 2013; Saługa et al., 2018). Within the genus Schistidium, this chorotype is represented by three species: S. falcatum, S. cupulare, and S. amblyophyllum.
Two species, Schistidium angustifolium and S. rivulariopsis, are Afro-American oreophytes. This distribution pattern is common among tropical mosses and liverworts and is exhibited by approximately 80 species occurring in the Andes and the mountains of East Africa (Frahm, 1982; Ochyra et al., 1992, 2002b, 2020; Ochyra & Ireland, 2004; Ellis et al., 2012a, 2014a, 2014b, 2014c, 2016a, 2016b).
Finally, two species, Schistidium andinum and S. praemorsum, represent the South American–Antarctic chorotypes. These species are widely distributed at high elevations along the Andes and extend southward into the northern maritime Antarctic region. This is a relatively rare distribution pattern, as many species in this group simultaneously exhibit Afro-American and amphi-Atlantic cool-temperate chorotypes on opposite shores of the Atlantic Ocean in mainland Africa and the Southern Ocean islands of the Kerguelen Province (Bednarek-Ochyra et al., 2000; Ochyra et al., 2008b).
. Conclusion
The rediscovery of Schistidium deguchianum in Jauja Province represents only the second documented locality of this poorly known Peruvian endemic. This new record extends the known range of this species by approximately 400 km northwest of the type locality and confirms its occurrence in the Central Andes at elevations above 3000 m. The discovery of this species in a historical herbarium collection originally assigned to another taxon highlights the importance of revising previously identified materials. Our assessment indicates that 20 Schistidium species are currently recognized in South America. Thirteen of these are comparatively well documented, whereas seven are known solely by their type collections and require critical taxonomic reassessment. The reinstatement of S. angustifolium and S. malacophyllum further demonstrates that species diversity in this region has previously been underestimated. Conversely, several Holarctic taxa traditionally reported from South America should be excluded from moss flora because the corresponding records are based on misidentified specimens. Chorological analysis revealed a predominance of Southern Hemisphere elements, including Andean endemics, Afro-American oreophytes, amphiatlantic cool-temperate species, and taxa shared between the Andes and maritime Antarctica. Only S. rivulare is a widespread bipolar element, emphasizing the distinct phytogeographical characteristics of South American Schistidium flora. Comprehensive revision of herbarium collections, combined with additional fieldwork and molecular studies, will therefore be essential for resolving taxonomy, true diversity, and distribution of the genus on the continent.
Acknowledgments
We are grateful to the Curators at B, BM, BR, FH, H, HBG, JE, MO, NY, PC, S and W for kindly allowing us to study their herbarium holdings of Schistidium. We would also like to thank the two anonymous reviewers for their careful reading of the manuscript and their insightful comments and helpful suggestions, which significantly improved its quality. The work of Ryszard Ochyra and Halina Bednarek-Ochyra was financially supported through the statutory fund of the W. Szafer Institute of Botany, Polish Academy of Sciences. The work of Vítězslav Plášek was carried out at MCBR UO (International Research and Development Center of the University of Opole), which was established as part of a project co-financed by the European Union under the European Regional Development Fund, RPO WO 2014–2020, Action 1.2 Infrastructure for R&D. Agreement No. RPOP.01.02.00-16-0001/17-00 dated January 31, 2018.